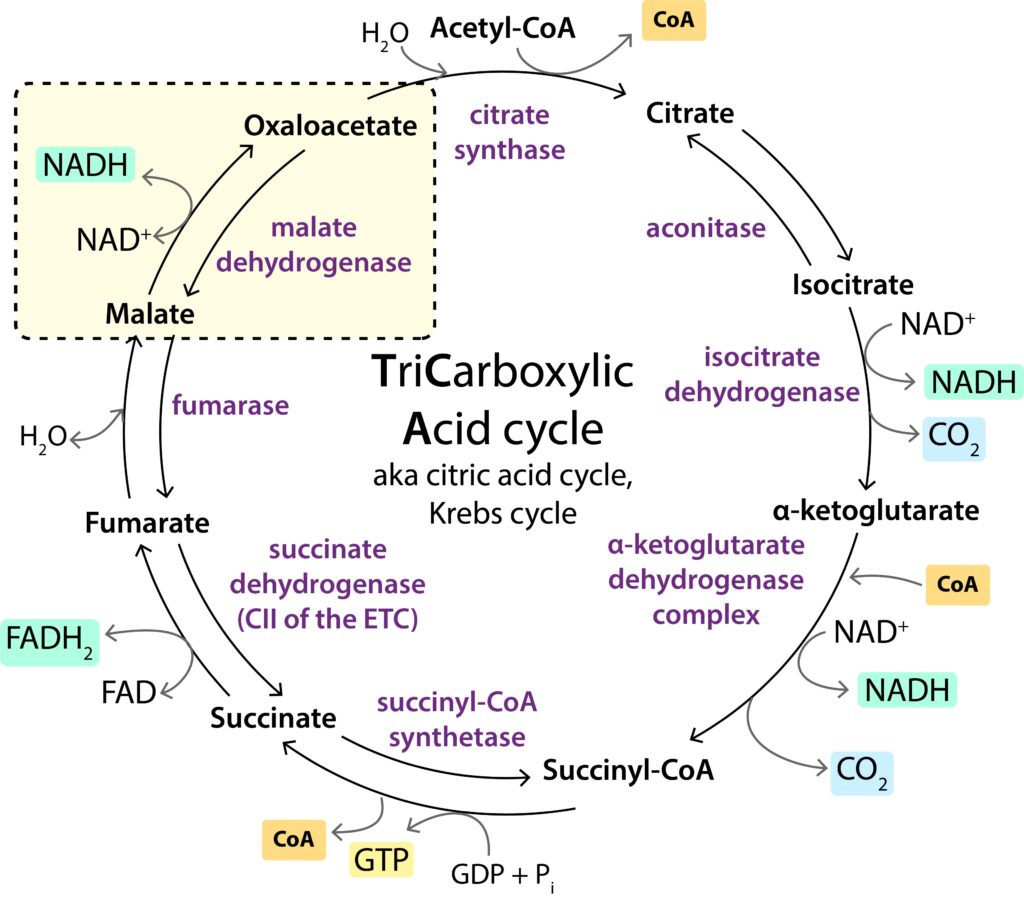
Our lab uses biochemistry and structural biology techniques to investigate unique and conserved features of metabolic enzymes from Bacillus bacteria capable of rewiring their metabolism to facilitate the process of “bioremediation” – using living organisms to clean up the environment. We’re most interested in the bioremediation of the toxic heavy metal chromium, Cr(VI), the core metabolic enzyme malate dehydrogenase (MDH)’s role in this process, and how the bacteria’s MDH is structurally well-suited for this task.
Our motivation
High levels of Cr(VI) are incompatible with most life. However, some bacteria are able to not only survive in its presence, but also reduce it to a much less hazardous form, Cr(III). A sort of biological “detox” if you will. This form of remediation is much more environmentally-friendly and sustainable than conventional chemical and physical methods.
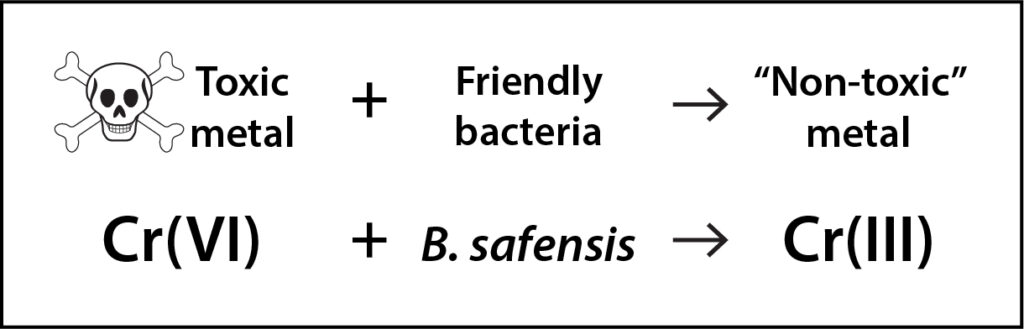
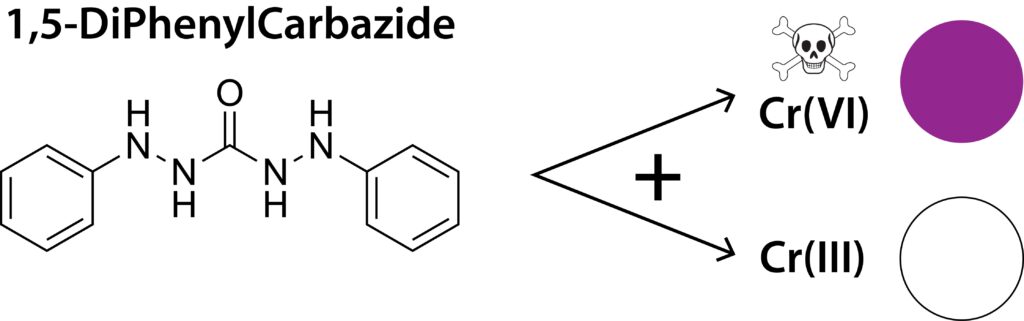
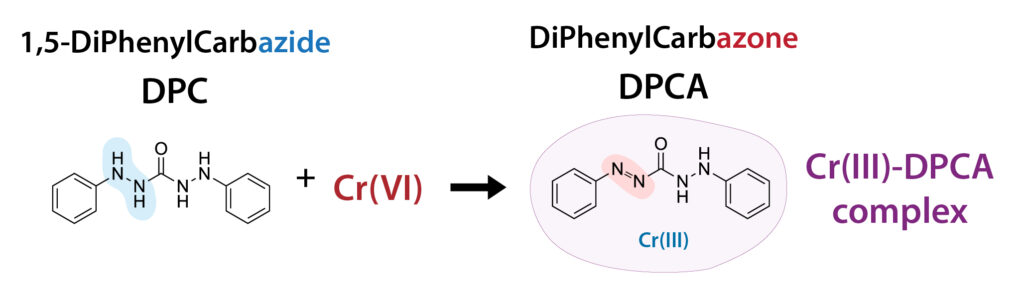
Through screening of a public culture collection, we identified uncharacterized strains of the friendly soil bacterium Bacillus safensis with this Cr(VI)-resisting and reducing superpower. We uncovered this superpower using a DPC (1,5-diphenylcarbazide)-based assay. “Assay” is just a fancy word for an experiment where you’re measuring something. And in this case, we were measuring Cr(VI) (that’s the bad stuff, remember). DPC reacts with Cr(VI) (but not Cr(III)) to form a purple complex. If we add Cr(VI) to the media (broth) the bacteria is growing in, and test the broth with the DPC assay, we will see a purple color unless the bacteria were able to reduce the Cr(VI). In such a case, the purple color would “disappear.” And this is what we found happen with our B. safensis strains.
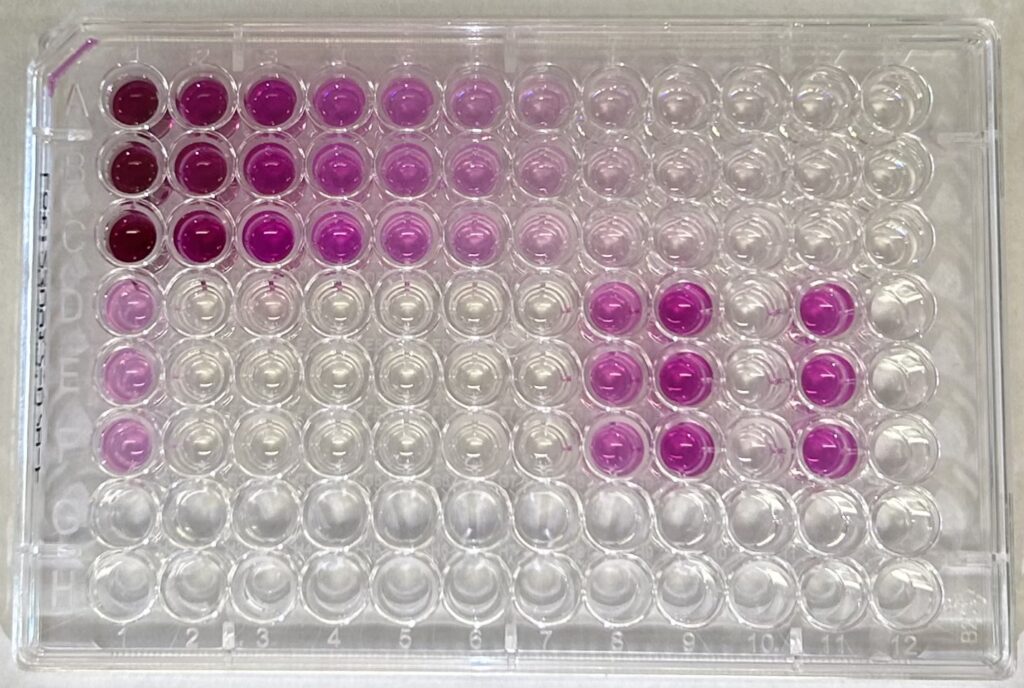
We were able to confirm, using atomic Emission Spectroscopy, that the total Cr levels remained unchanged, indicating that the toxic Cr(VI) was chemically reduced to the non-toxic Cr(III).
Now, we’re starting to look under the hood (or I guess under the cell wall would be more precise) metabolically in order to figure out how these bacteria rewire their metabolism during the process.
Malate Dehydrogenase (MDH)
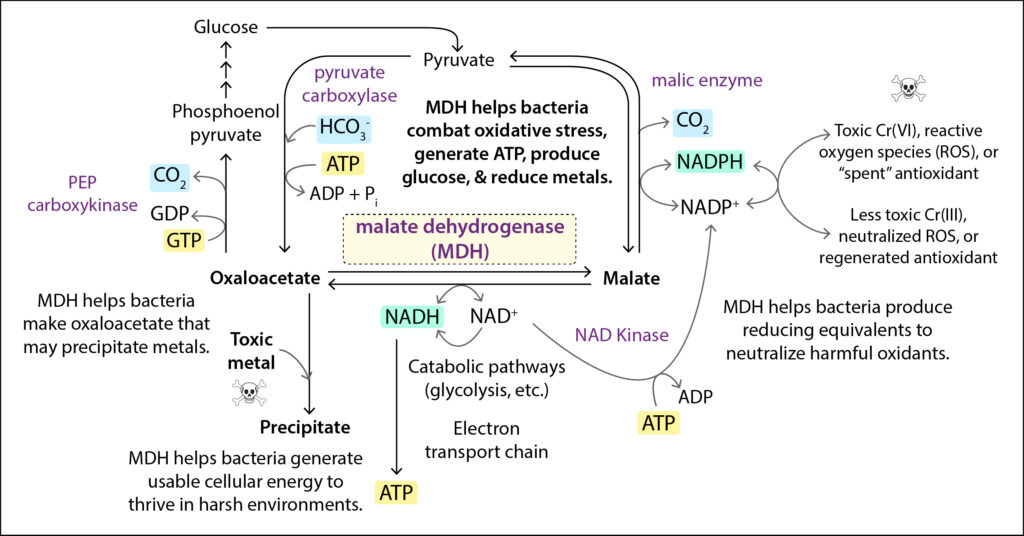
The focal point of our investigation is the enzyme malate dehydrogenase (MDH), which plays a core role in central metabolism. It serves as a sort of coordinating hub whose activities and interactions can help direct carbon metabolism to meet the need for energy, the need for metal-chelating metabolites, and the need for reducing equivalents to counteract reactive oxygen species (ROS) generated by metal stress.
In vitro and in silico analysis
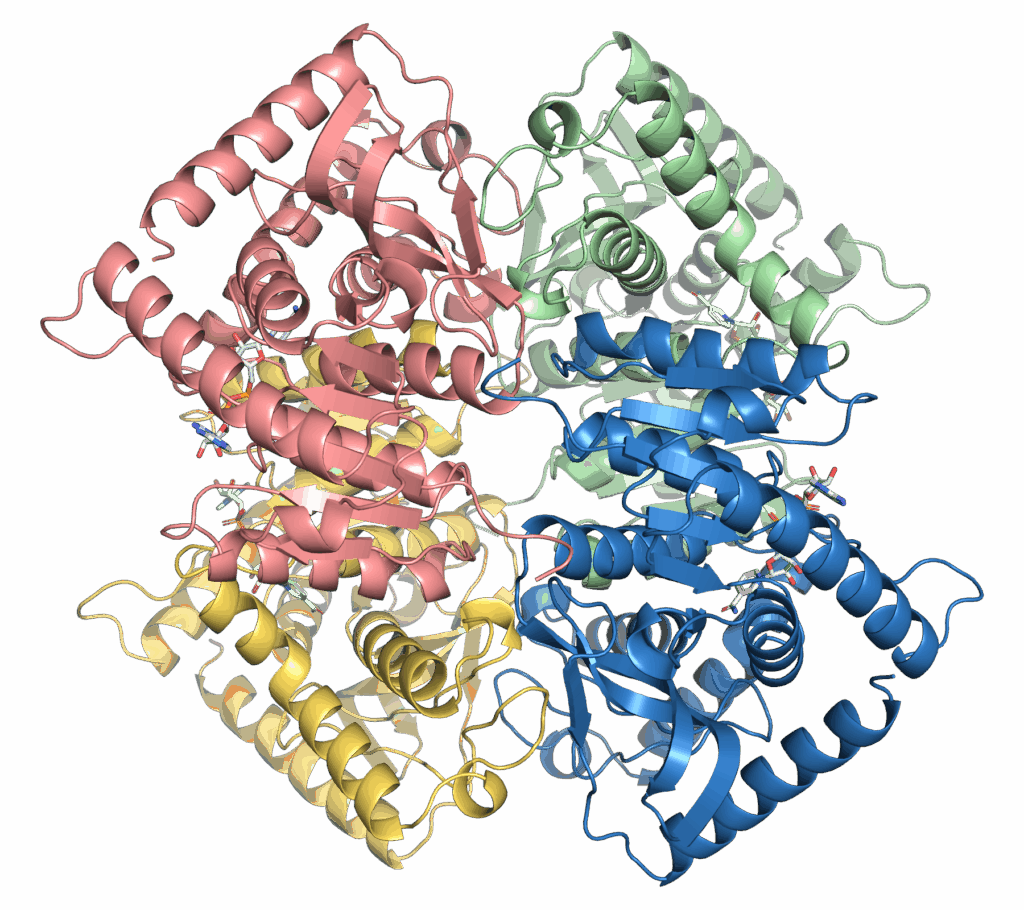
Very little is known about Bacillus safensis MDH, but it is part of an underexplored, yet fascinating, evolutionary branch of MDH enzymes called LDH-like MDH’s. These LDH-like MDH’s possess intriguing, potentially exploitable, structural and enzymatic features–most notably a tetrameric (4 subunit) structure not found in the MDH proteins of animals and plants. There remain many outstanding questions about if and how the subunits communicate with one another and what functional implications such communication brings. Exploring B. safensis MDH, and MDH from the related widely-used model organism B. subtilis therefore offers important insight into both fundamental and applied biochemistry.
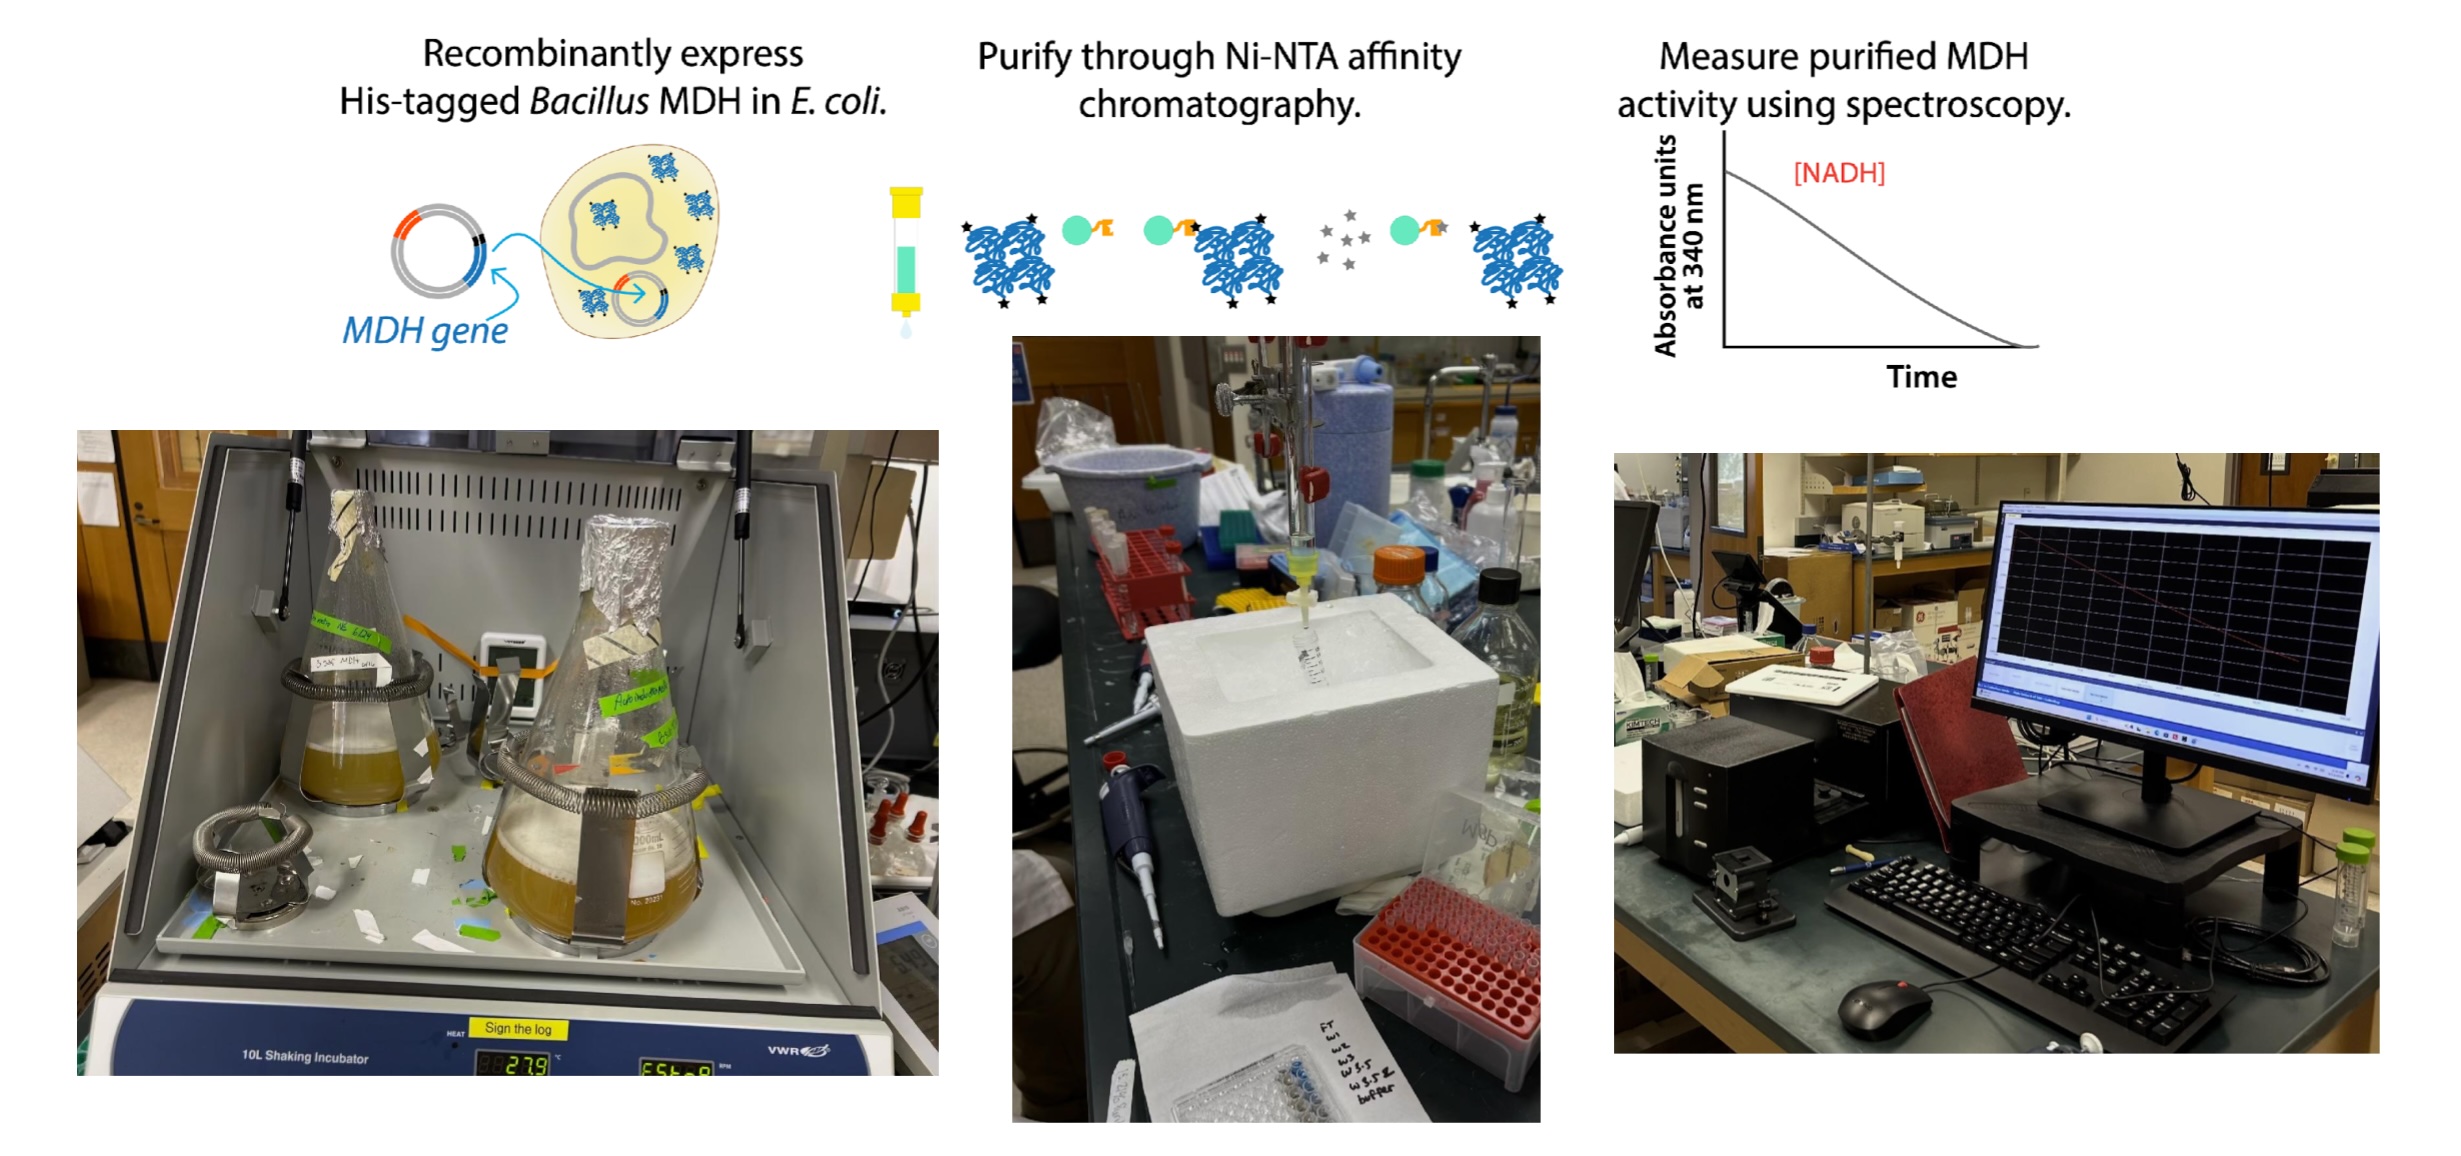
Through recombinant protein expression, we get (harmless) E. coli cells to make a lot of the Bacillus safensis and Bacillus subtilis MDH proteins, which we then purify. Then we can test their activity using an MDH enzymatic assay and their structural dynamics using biophysical assays (Differential Scanning Fluorimetry (DSF), Circular Dichroism (CD), Size Exclusion Chromatography – Small Angle X-ray Scattering (SEC-SAXS), etc.). Having the pure protein lets us manipulate conditions to test its limits and see how it’s affected by its environment such as pH, temperature, even the presence of metals. We can even make changes to the proteins’ sequences to tease apart how they work.
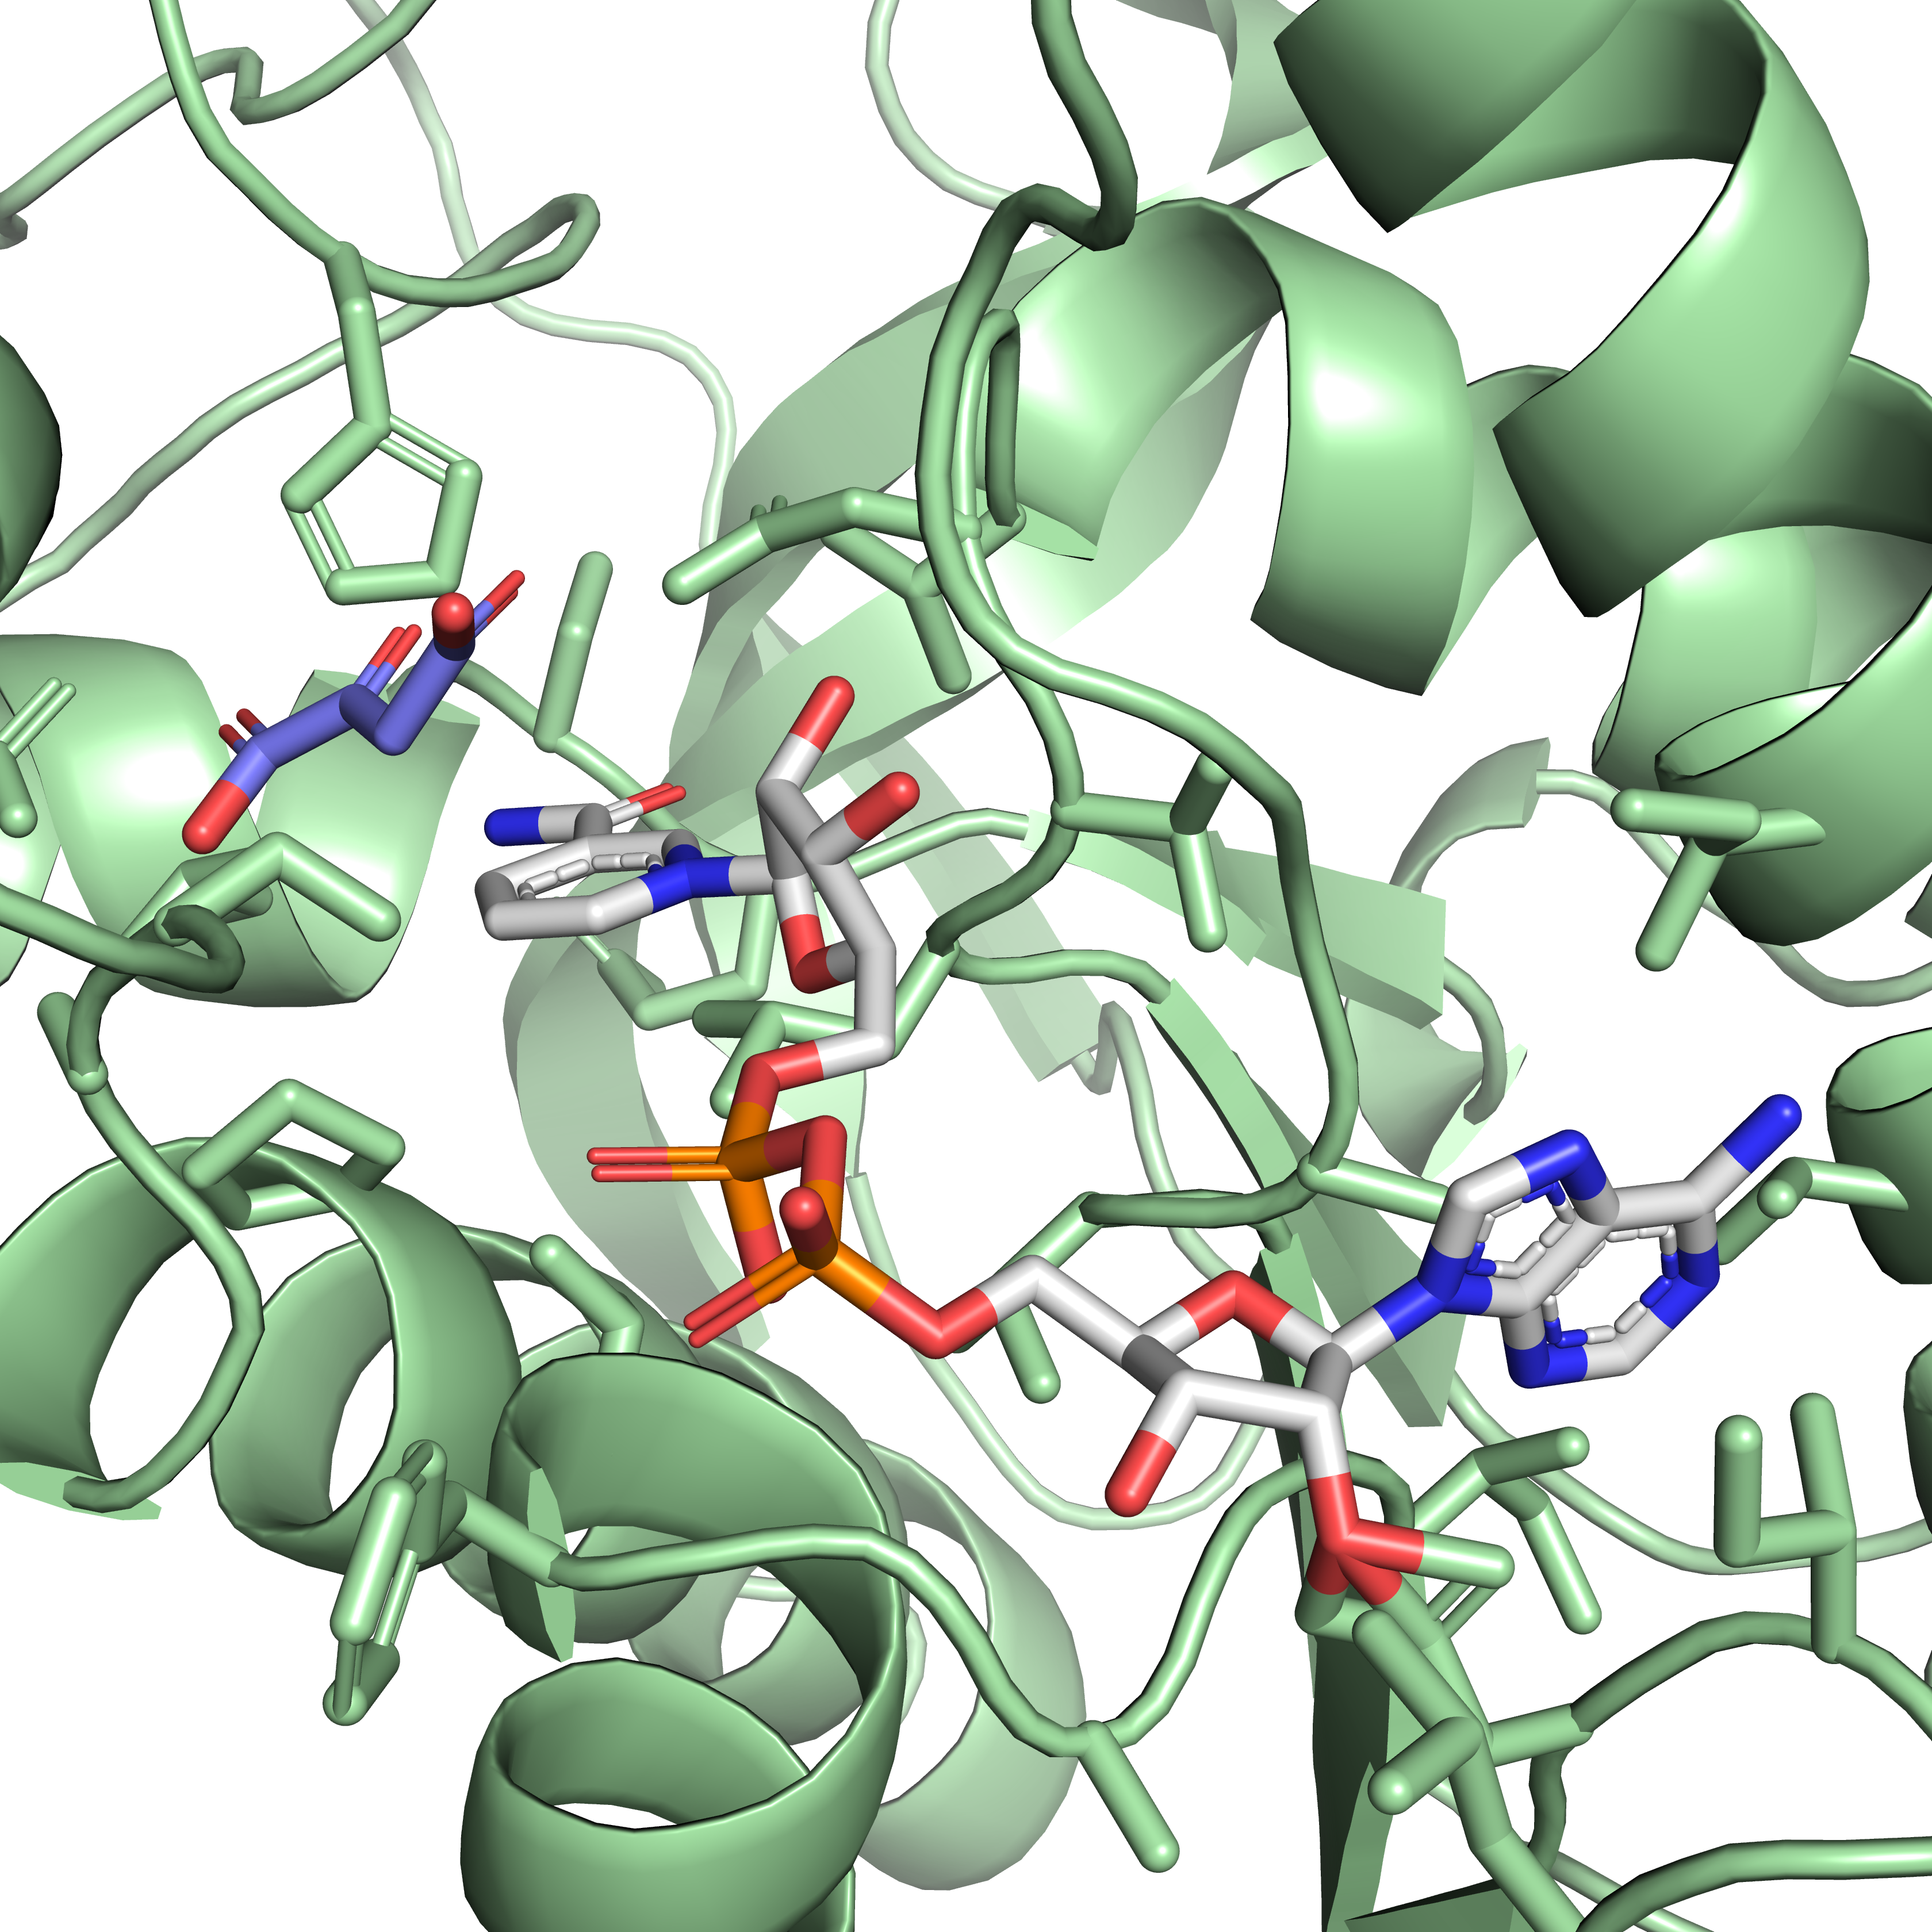
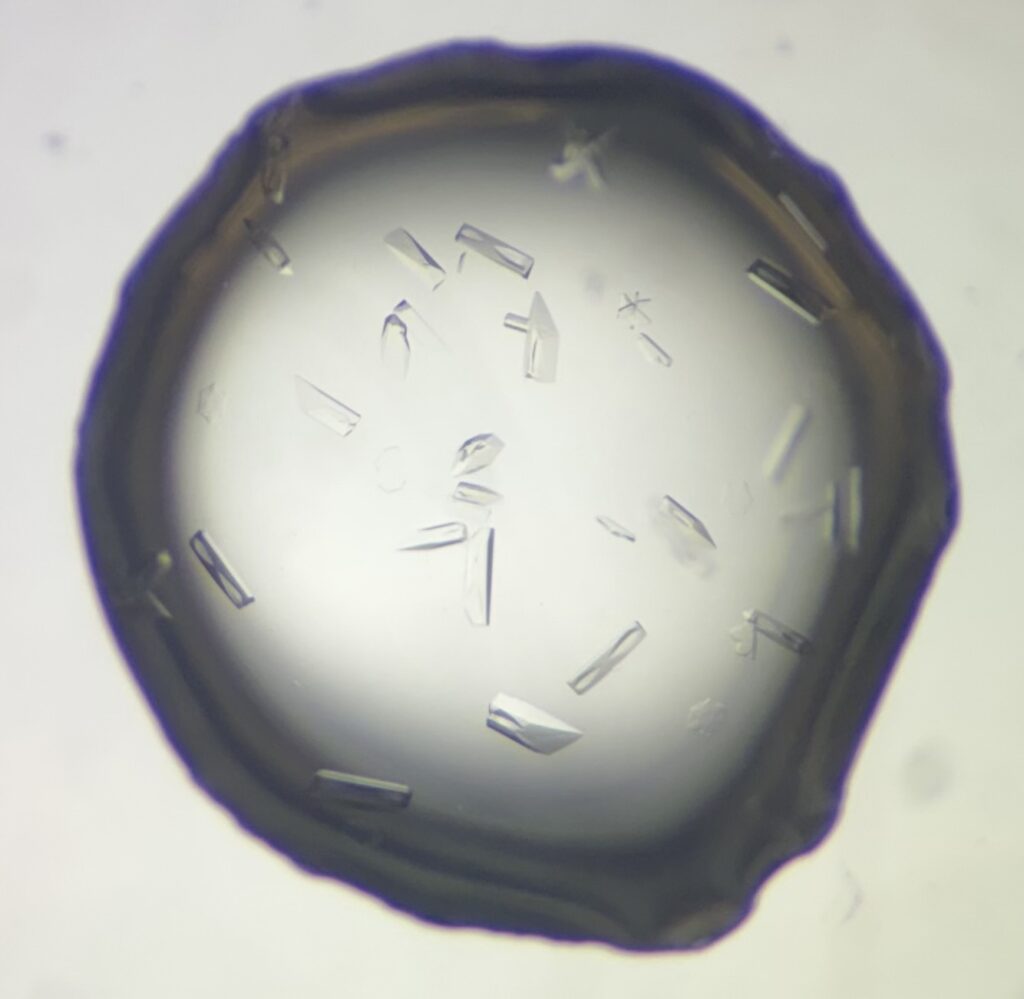
We use structural biology techniques including x-ray crystallography and complementary “in silico” computational methods (structural modeling and docking, molecular dynamics, conservational analysis, etc.) to gain further insights into specific structural adaptations at the root of the phenomena we observe.
We can combine experimental structural data with in silico predictions to rationally design and introduce mutations to the proteins to study their effects. One aspect we are exploring with such “protein engineering” is the multimerization status of the protein (assessed using techniques including size exclusion chromatography) and its implications for activity (assessed using enzyme assays). We are also exploring the structural roots of pH-dependent phenomena we have discovered.
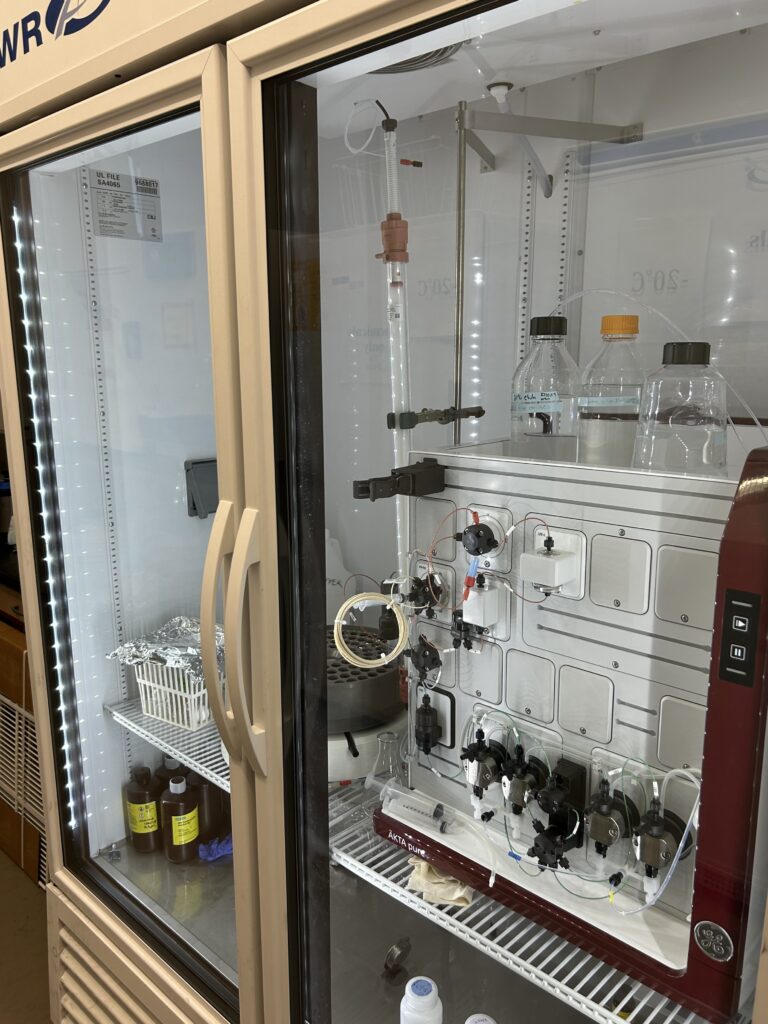
Through this combination of strategies, we can characterize kinetic, structural, and regulatory properties of Bacillus safensis MDH that allows for metabolic adaptation to harsh environments.
Most of the experiments are carried out in-house, but the Bibel lab is also collaborative. Bri believes that collaboration is crucial for scientific progress and tap into the Malate Dehydrogenase CUREs Community (MCC) to expand the scope of research we can perform. Some of the computational work, in addition to the SEC-SAXS is carried out in close collaboration with Chris Berndsen’s lab at James Madison University, but Bibel Lab students are deeply involved in the process, exposing them to new techniques and skills.
In vivo exploration
In vitro and in silico (on a computer) are great for that sorts of things, but not very realistic. Therefore, back at the organismal level, we plan to compare the metabolism of different strains and bacterial species in the presence of metals, using analytical methods like GC-MS (Gas Chromatography-Mass Spectrometry) to measure intracellular metabolites, HPLC (High Pressure Liquid Chromatography) to measure secreted metabolites, and infrared (IR) spectroscopy to investigate cellular composition. We can compare changes in metabolites as well as MDH activity to Bacillus strains exposed to various stressors (Cr(VI), other heavy metals, other oxidatants, etc.) to determine what changes might be stressor-specific. And try to correlate any differences we see between strains to differences in the strains’ genomes.
We’re also doing some genetic engineering to investigate the role of MDH in vivo (e.g. with MDH knockout strains) and test our in silico and in vitro findings in the context of bioremediation. For example, we can use molecular modeling to make predictions about the functional roles of particular amino acids, change those amino acids in our recombinant MDH using site-directed mutagenesis, and test the results in enzyme assays and other in vitro experiments. If we see effects, we can then use homologous recombination techniques to introduce those mutations into the Bacillus safensis genome(s) to determine in vivo effects.
The big picture
With these experiments, we seek to tease apart both conserved and unique adaptations of B. safensis metabolic enzymes. We hope to put this knowledge to practical use by optimizing the bioremediation potential of Bacillus safensis with the goal of using it to clean up heavy metal-contaminated environments and promote the growth of plants in once-barren landscapes. At the same time, we aim to elucidate structure-function relationships of multimeric proteins, providing valuable training data for the next generation of computer software capable of more accurately predicting and designing the proteins of the future.
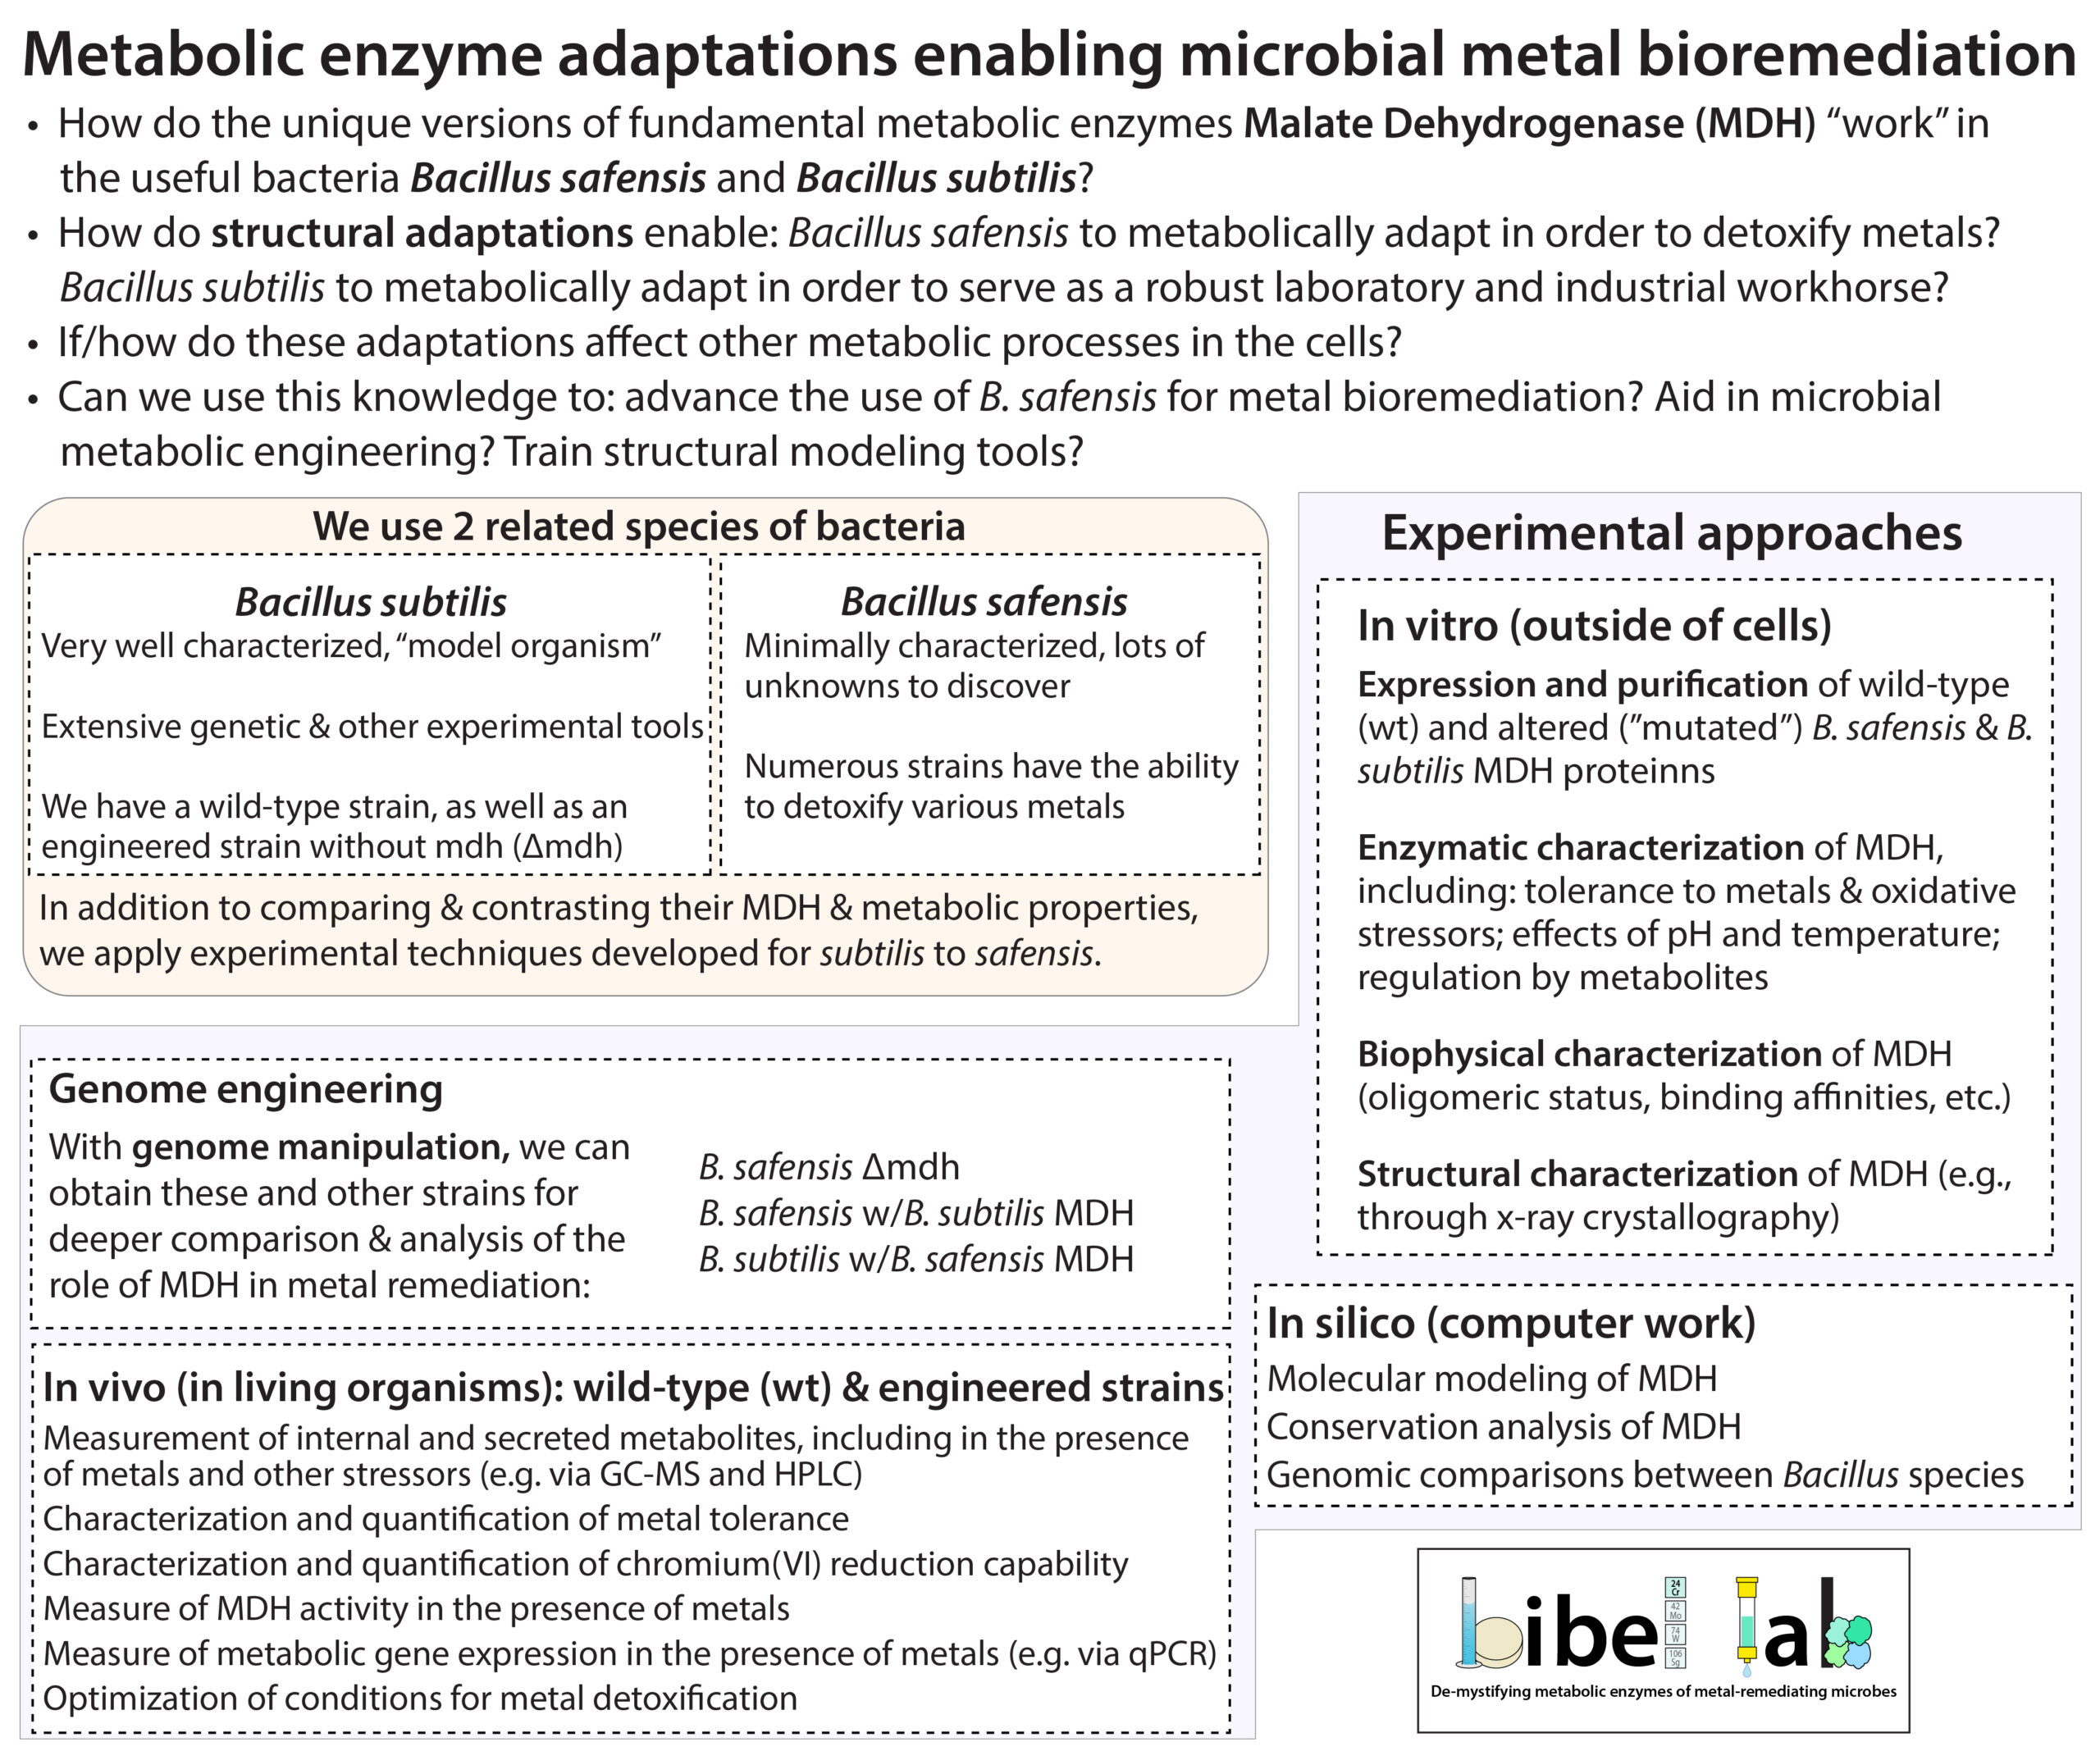
Our work is undergraduate–driven and I’m so proud of the student researchers I have the privilege of working with!
Publications and preprints
Biophysical and enzymatic comparison of Bacillus safensis and Bacillus subtilis malate dehydrogenase (MDH) enzymes
Haley R Zafiropoulo, Juliette E Thomas, Nicholas R Cortez, Korina Apostol, Alice de Sá, Ryan Khosravi, Liam Moore, Christopher E Berndsen, Brianna Bibel
bioRxiv 2026.05.13.723581; doi: https://doi.org/10.64898/2026.05.13.723581